For laboratory research only. Not for human or animal use. This article gives no dosing, administration or therapeutic advice.
Short answer: thymosin alpha-1 and LL-37 are both naturally occurring human peptides studied for their effects on immunity, but they work at different layers of it. Thymosin alpha-1 is a thymic peptide, the first biologically active peptide isolated and sequenced from the thymic preparation thymosin fraction 5 [1]. Its best-described action is on dendritic cells, which it primes through Toll-like receptor signalling [2][3]. LL-37 is the only human cathelicidin, a 37-residue fragment cut from the protein hCAP18 [4][5]. It kills microbes directly by disrupting their membranes [6] and also acts as a chemoattractant through the receptor FPRL1 [4]. One is a signal to antigen-presenting cells; the other is an effector molecule that does some of the defending itself.
Identity at a glance
Formula and mass values are from PubChem.
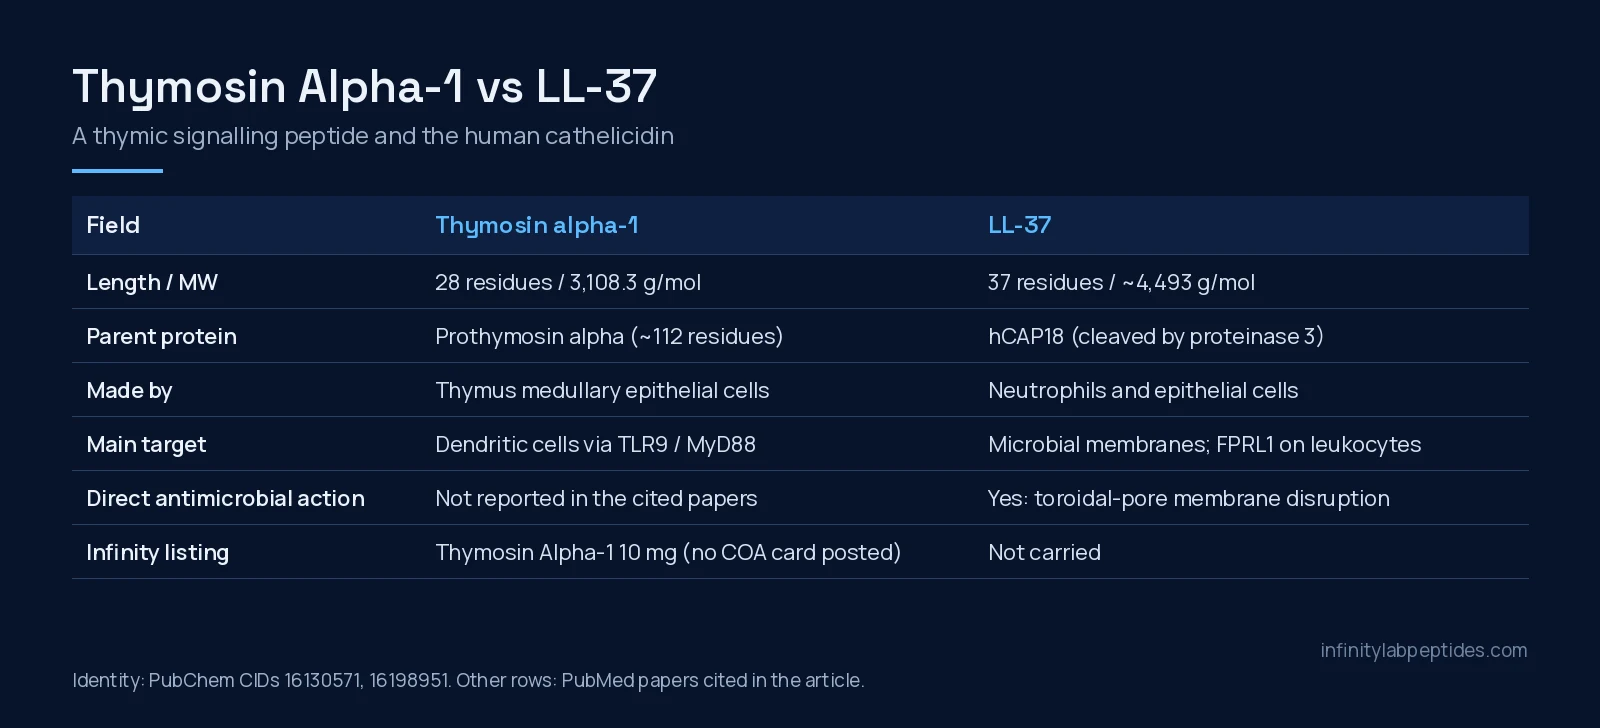
| Field | Thymosin alpha-1 | LL-37 |
|---|---|---|
| Other names (PubChem) | Thymalfasin, Zadaxin | Cathelicidin LL-37, hCAP18 fragment, ropocamptide |
| Length | 28 residues, N-terminally acetylated | 37 residues, beginning with two leucines (hence “LL”) |
| Molecular formula | C129H215N33O55 | C205H340N60O53 |
| Molecular weight | 3,108.3 g/mol | about 4,493 g/mol |
| CAS (PubChem synonym) | 62304-98-7 | 154947-66-7 |
| PubChem CID | 16130571 | 16198951 |
| Parent protein | Prothymosin alpha (about 112 residues) [7] | hCAP18 [5] |
| Where it is made | Thymus medullary epithelial cells [1] | Neutrophils and various epithelial cells [4] |
| Main receptor or target | Toll-like receptor signalling (TLR9 / MyD88) in dendritic cells [8][3] | Microbial membranes; FPRL1 on leukocytes [6][4] |
Where each one comes from
Thymosin alpha-1: a fragment of prothymosin alpha
Thymosin alpha-1 was first purified from thymosin fraction 5, a partially purified calf thymus preparation, and a 1987 monoclonal antibody study located its production to the epithelial cells of the thymic medulla [1]. When a Roche group used an antibody against synthetic thymosin alpha-1 to look for it in rat thymus, the main immunoreactive substance was not the 28-residue peptide but a larger polypeptide of about 112 residues carrying the thymosin alpha-1 sequence at its N-terminus. They named it prothymosin alpha [7]. In that study, free thymosin alpha-1 itself was not detected in the extracts [7], which is worth remembering when reading older work that measured “thymosin alpha-1” by immunoassay.
LL-37: cut from hCAP18 after release
Cathelicidins are proteins stored in neutrophil granules whose active part is a C-terminal peptide that has to be cleaved off. In cattle and pigs elastase does the cutting. A 2001 study of human neutrophils found that hCAP18, the only human cathelicidin, was not cleaved inside cells after phagocytosis; it was cut to LL-37 in exocytosed material, and of the three serine proteases from azurophil granules, proteinase 3 alone was responsible [5]. LL-37 is also made by various epithelial cells, not only by neutrophils [4].
How each one works
Thymosin alpha-1 talks to dendritic cells
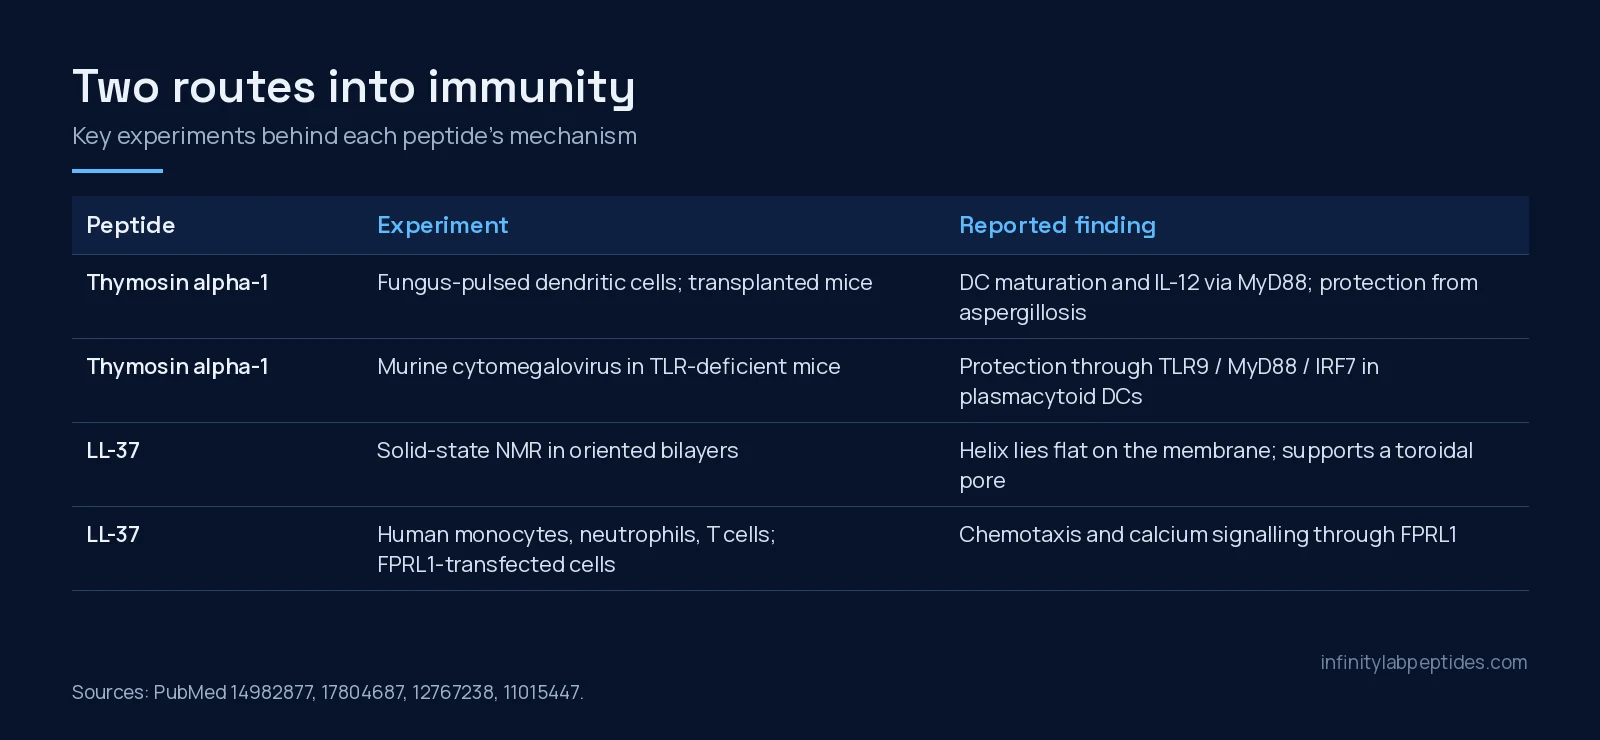
Much of the modern mechanistic picture comes from Romani, Garaci and colleagues. In a 2004 study, thymosin alpha-1 induced maturation and interleukin-12 production in fungus-pulsed dendritic cells through a p38 MAPK and NF-kappaB pathway that depended on MyD88 and involved distinct Toll-like receptors. In mice given haematopoietic transplants, the synthetic peptide activated Th1-dependent antifungal immunity, sped myeloid recovery and protected against aspergillosis [2].
Two follow-ups sharpened this. In mouse cytomegalovirus infection, thymosin alpha-1 protected both susceptible and resistant mice, and its effect ran through TLR9, MyD88 and IRF7 [8]. A 2006 study showed the other side of TLR9 signalling: thymosin alpha-1 induced the tryptophan-catabolising enzyme IDO in dendritic cells, which required TLR9 and type I interferon receptor signalling and produced interleukin-10 and regulatory T cells [3]. So the same peptide was reported to support both priming and tolerance, depending on the dendritic cell subset.
LL-37 acts on membranes and on leukocytes
LL-37 is an amphipathic alpha-helix. Solid-state NMR in oriented lipid bilayers showed the helix lying parallel to the membrane surface, which ruled out a barrel-stave pore; the absence of micelle formation ruled out a detergent-like mechanism; and the induced positive curvature strain supported a toroidal pore model of membrane disruption [6]. In detergent micelles, LL-37 adopts a helix-break-helix structure with unstructured termini [9]. A 2016 review describes it as a pore-forming antibacterial peptide that also forms oligomers under physiological conditions, and links those oligomers to some of its cytotoxic and immunomodulatory effects [10].
Beyond killing microbes, LL-37 recruits cells. It is chemotactic for human monocytes, neutrophils and T lymphocytes, and it signals through formyl peptide receptor-like 1 (FPRL1), shown in FPRL1-transfected HEK293 cells and by cross-desensitisation with an FPRL1-specific agonist [4]. A 2015 review lists antibiofilm, antiviral and antiparasitic activity alongside roles in angiogenesis, wound healing and apoptosis [11]. Not every effect runs through FPRL1: LL-37 inhibited HIV-1 replication in blood mononuclear cells and CD4+ T cells in vitro by a route shown to be independent of FPRL1 signalling [12].
Side by side: what kind of research each suits
The overlap is narrower than the “immune peptide” label suggests. Thymosin alpha-1 has no reported direct antimicrobial membrane activity in these papers; its effects in infection models came through the host’s dendritic cells and T cells [2][8]. LL-37, by contrast, acts directly on microbes and also directly on host leukocytes [6][4].
Regulatory context
A 2007 paper describes thymosin alpha-1 as approved for treatment of some viral infections and as an immune adjuvant [8], and a 2001 pharmacy review noted Phase III trials in hepatitis C at that time [13]. A 2020 literature review and a 2025 review on ageing summarise its broader clinical history and the interest in thymic involution [14][15]. We mention this as background only. LL-37 is a research peptide in the papers cited here. Both peptides as we discuss them are for laboratory research and are not drug products.
Gaps worth knowing
- Immunoassay identity. Antibodies to thymosin alpha-1 cross-react with prothymosin alpha, which was the main immunoreactive form in rat thymus [7]. Mass spectrometry avoids that ambiguity.
- Context-dependent immune effects. Thymosin alpha-1 drove both Th1 priming and IDO-mediated tolerance in different dendritic cell settings [2][3]. Results depend on cell subset and stimulus.
- Oligomerisation of LL-37. LL-37’s tendency to oligomerise affects how it binds surfaces [10], so buffer, concentration and serum content can change assay outcomes.
- Membrane composition. Lipid type, charge and cholesterol changed how much LL-37 perturbed model bilayers [6].
Sourcing thymosin alpha-1 for laboratory work
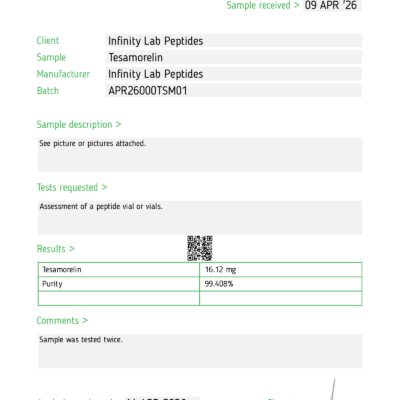
Our Thymosin Alpha-1 10 mg listing is supplied for in vitro and laboratory research only; we do not currently carry LL-37. At the time of writing our COA page lists no certificate for Thymosin Alpha-1, so we do not quote a purity figure, batch or date for it. For neighbouring comparisons, see thymosin alpha-1 vs KPV and TB-500 vs thymosin beta-4, which explains how the beta-thymosins differ from thymosin alpha-1 despite the shared name. You can also buy research peptides in Canada from Infinity Lab Peptides.
Frequently asked questions
What is the difference between thymosin alpha-1 and LL-37?
Thymosin alpha-1 is a 28-residue thymic peptide whose best-described action is priming dendritic cells through Toll-like receptor signalling. LL-37 is the 37-residue human cathelicidin, cut from hCAP18; it disrupts microbial membranes directly and recruits leukocytes through the receptor FPRL1.
Is LL-37 an antibiotic and thymosin alpha-1 not?
In the cited research, yes in effect. LL-37 kills microbes by disrupting their membranes, consistent with a toroidal pore model. Thymosin alpha-1’s effects in infection models ran through the host’s dendritic cells and T cells rather than direct action on the microbe.
Where do the two peptides come from in the body?
Thymosin alpha-1 is made by thymic medullary epithelial cells and is the N-terminal part of a larger protein, prothymosin alpha. LL-37 is released from hCAP18 by proteinase 3 after neutrophil granule contents are exocytosed, and it is also made by epithelial cells.
Is thymosin alpha-1 related to thymosin beta-4 or TB-500?
Only by name. Thymosin alpha-1 comes from prothymosin alpha, while thymosin beta-4 belongs to the separate beta-thymosin family; TB-500 is a research peptide based on thymosin beta-4.
Does Infinity Lab Peptides post a COA for Thymosin Alpha-1?
Not at the time of writing. Our COA page lists no certificate for Thymosin Alpha-1 10 mg, so we do not quote a purity figure, batch or date. We do not carry LL-37.
References
- Oates KK, Naylor PH, Goldstein AL (1987). Localization of thymosin alpha 1 production to thymus medullary epithelial cells by use of monoclonal antibodies. Hybridoma. PMID: 2445653. doi: 10.1089/hyb.1987.6.47.
- Romani L, Bistoni F, Gaziano R et al. (2004). Thymosin alpha 1 activates dendritic cells for antifungal Th1 resistance through toll-like receptor signaling. Blood. PMID: 14982877. doi: 10.1182/blood-2003-11-4036.
- Romani L, Bistoni F, Perruccio K et al. (2006). Thymosin alpha1 activates dendritic cell tryptophan catabolism and establishes a regulatory environment for balance of inflammation and tolerance. Blood. PMID: 16741252. doi: 10.1182/blood-2006-02-004762.
- De Yang, Chen Q, Schmidt AP et al. (2000). LL-37, the neutrophil granule- and epithelial cell-derived cathelicidin, utilizes formyl peptide receptor-like 1 (FPRL1) as a receptor to chemoattract human peripheral blood neutrophils, monocytes, and T cells. J Exp Med. PMID: 11015447. doi: 10.1084/jem.192.7.1069.
- Sørensen OE, Follin P, Johnsen AH et al. (2001). Human cathelicidin, hCAP-18, is processed to the antimicrobial peptide LL-37 by extracellular cleavage with proteinase 3. Blood. PMID: 11389039. doi: 10.1182/blood.v97.12.3951.
- Henzler Wildman KA, Lee DK, Ramamoorthy A (2003). Mechanism of lipid bilayer disruption by the human antimicrobial peptide, LL-37. Biochemistry. PMID: 12767238. doi: 10.1021/bi0273563.
- Haritos AA, Goodall GJ, Horecker BL (1984). Prothymosin alpha: isolation and properties of the major immunoreactive form of thymosin alpha 1 in rat thymus. Proc Natl Acad Sci U S A. PMID: 6583693. doi: 10.1073/pnas.81.4.1008.
- Bozza S, Gaziano R, Bonifazi P et al. (2007). Thymosin alpha1 activates the TLR9/MyD88/IRF7-dependent murine cytomegalovirus sensing for induction of anti-viral responses in vivo. Int Immunol. PMID: 17804687. doi: 10.1093/intimm/dxm097.
- Porcelli F, Verardi R, Shi L et al. (2008). NMR structure of the cathelicidin-derived human antimicrobial peptide LL-37 in dodecylphosphocholine micelles. Biochemistry. PMID: 18439024. doi: 10.1021/bi702036s.
- Xhindoli D, Pacor S, Benincasa M et al. (2016). The human cathelicidin LL-37–A pore-forming antibacterial peptide and host-cell modulator. Biochim Biophys Acta. PMID: 26556394. doi: 10.1016/j.bbamem.2015.11.003.
- Bandurska K, Berdowska A, Barczyńska-Felusiak R et al. (2015). Unique features of human cathelicidin LL-37. Biofactors. PMID: 26434733. doi: 10.1002/biof.1225.
- Bergman P, Walter-Jallow L, Broliden K et al. (2007). The antimicrobial peptide LL-37 inhibits HIV-1 replication. Curr HIV Res. PMID: 17627504. doi: 10.2174/157016207781023947.
- Ancell CD, Phipps J, Young L (2001). Thymosin alpha-1. Am J Health Syst Pharm. PMID: 11381492. doi: 10.1093/ajhp/58.10.886.
- Dominari A, Hathaway Iii D, Pandav K et al. (2020). Thymosin alpha 1: A comprehensive review of the literature. World J Virol. PMID: 33362999. doi: 10.5501/wjv.v9.i5.67.
- Simonova MA, Ivanov I, Shoshina NS et al. (2025). Aging and Thymosin Alpha-1. Int J Mol Sci. PMID: 41373628. doi: 10.3390/ijms262311470.